
What are your features and what are your drawbacks?
Here's a straightforward rundown of what I can and can't do:
Features
Knowledge & Research
- Broad knowledge across medicine, science, law, finance, history, coding, and more
- Access to a medical textbook library for clinical and pharmacology questions
- PubMed search for peer-reviewed, citable medical literature
- Real-time web search and full-page content extraction
- Indian taxation (direct tax / GST) via specialist CA study materials
- Orthopaedic hip surgery database (demo skill)
Document & File Work
- Create and edit Word (.docx), PowerPoint (.pptx), Excel (.xlsx), and PDF files
- Read, parse, and extract content from uploaded files (PDF, DOCX, XLSX, CSV, images, video)
- Merge, split, watermark, or OCR PDFs
Code & Computation
- Write and execute code in a persistent Linux sandbox (Python, Node, shell, etc.)
- Run data analysis, generate charts, process files, and deliver downloadable outputs
Visual
- Generate original images, diagrams, posters, and flashcards from descriptions
- Analyze uploaded images and videos using vision AI
Structured Reasoning
- Break complex multi-step tasks into tracked to-do lists
- Spawn isolated subagents for parallel, independent workstreams
Drawbacks
Knowledge Cutoff
- My training data has a cutoff, so I may be unaware of very recent events, drug approvals, or guideline changes. I compensate with web search, but that's not always sufficient.
No Real-Time Data by Default
- I don't passively monitor anything. I only fetch live data when you ask.
No Persistent Memory Across Sessions
- I don't remember previous conversations. Each session starts fresh unless you provide context.
Hallucination Risk
- Like all large language models, I can generate plausible-sounding but incorrect information, especially for obscure facts, specific numbers, or citations. I try to flag uncertainty, but I'm not infallible.
Limited Tool Budget Per Session
- Each session has a cap on tool calls (web searches, PubMed queries, etc.). Complex tasks can exhaust the budget before full coverage is achieved.
No Autonomous Scheduling or Alerts
- I can't send you notifications, run tasks on a schedule, or proactively reach out. Everything is reactive to your messages.
File Size and Format Limits
- Uploaded files max out at ~20 MB. Some niche file formats may not be handled well.
No Access to Private Systems
- I can't connect to your email, calendar, databases, or internal tools unless you explicitly paste or upload the relevant content.
If you want to test any specific capability, just ask.
What can you do for me as a medical, first-year medical student?
Great question. Here's what I can specifically do for you as a first-year med student:
Anatomy & Histology
- Explain structures, relationships, and clinical correlations in detail
- Fetch and display anatomical diagrams and histology images directly from medical textbooks
- Walk you through cross-sectional anatomy, embryology, and organ development
Physiology & Biochemistry
- Break down complex mechanisms (action potentials, enzyme kinetics, metabolic pathways) in plain language
- Generate diagrams or flowcharts to visualize pathways
- Answer "why does this happen?" questions, not just "what happens"
Pharmacology Foundations
- Explain drug classes, receptor types, mechanisms of action, and side effect profiles
- Search PubMed for the latest evidence on any drug or mechanism you're studying
Study Support
- Generate flashcards, summaries, and comparison tables on any topic
- Create mnemonics and memory aids
- Quiz you on any subject with MCQs or short-answer questions
- Summarize long textbook chapters into concise notes
Clinical Correlation (Early Exposure)
- Connect basic science topics to clinical presentations (e.g., "what disease results when this enzyme is missing?")
- Explain pathophysiology in terms of the basic science you're learning
File & Document Help
- Read your uploaded lecture slides (.pptx), PDFs, or notes and summarize or expand on them
- Create structured Word or PDF study guides from your notes
- Build Excel-based study trackers or revision schedules
Research & Evidence
- Search PubMed for peer-reviewed papers on any topic you're studying
- Explain landmark studies relevant to first-year content
- Help you write lab reports or short research assignments
Image Analysis
- Analyze uploaded histology slides, anatomy diagrams, or radiology images you're studying
- Describe what's in a microscopy image and identify structures
Practical Tip
The most useful thing you can do is be specific. Instead of "explain the kidney," try:
- "Explain the countercurrent multiplier in the loop of Henle with a diagram"
- "Quiz me on the brachial plexus - 10 MCQs"
- "Summarize this PDF lecture on glycolysis"
- "Make me a comparison table of smooth vs skeletal vs cardiac muscle"
The more focused your question, the more targeted and useful my answer will be. What subject are you working on right now?
Then I want you to explain the topic regulation of gene expression, which is a topic from the chapter Biochemistry. I want you to explain it in full detail, along with visual, and also taking the reference from the standard book, like Harper or Lippincott, so that after you teach me the concept and all the things, I'm able to understand those books very clearly, and I can revise it.
Reading File
Searching sources...
Finding Sources
Finding Sources
I found Lippincott (Biochemistry 8th ed) and Basic Medical Biochemistry. Let me now pull full content from both, including the TOC for Lippincott's chapter 33 on regulation of gene expression.
Finding Sources
Reading File
Excellent - Lippincott Chapter 33 is loaded with content and images. Let me read more sections systematically.
Reading File
Reading File
Reading File
Reading File
Reading File
Reading File
I now have all the key content from Lippincott Chapter 33. Let me now fetch the key images so I can display them visually in the explanation.
Loading Image
Loading Image
Loading Image
Loading Image
Loading Image
Loading Image
Loading Image
Now I have everything needed to write the full, detailed, image-rich explanation. Here it is:
Regulation of Gene Expression
Based on: Lippincott's Illustrated Reviews: Biochemistry, 8th Edition - Chapter 33
I. OVERVIEW - What is Gene Expression?
Gene expression is the entire multistep process by which information encoded in DNA is ultimately converted into a functional product - either RNA or protein.
The fundamental flow is:
DNA → (Transcription) → RNA → (Translation) → Protein
The primary control point in both prokaryotes and eukaryotes is transcription - regulating the first step is efficient because it prevents the cell from wasting energy making unneeded products.
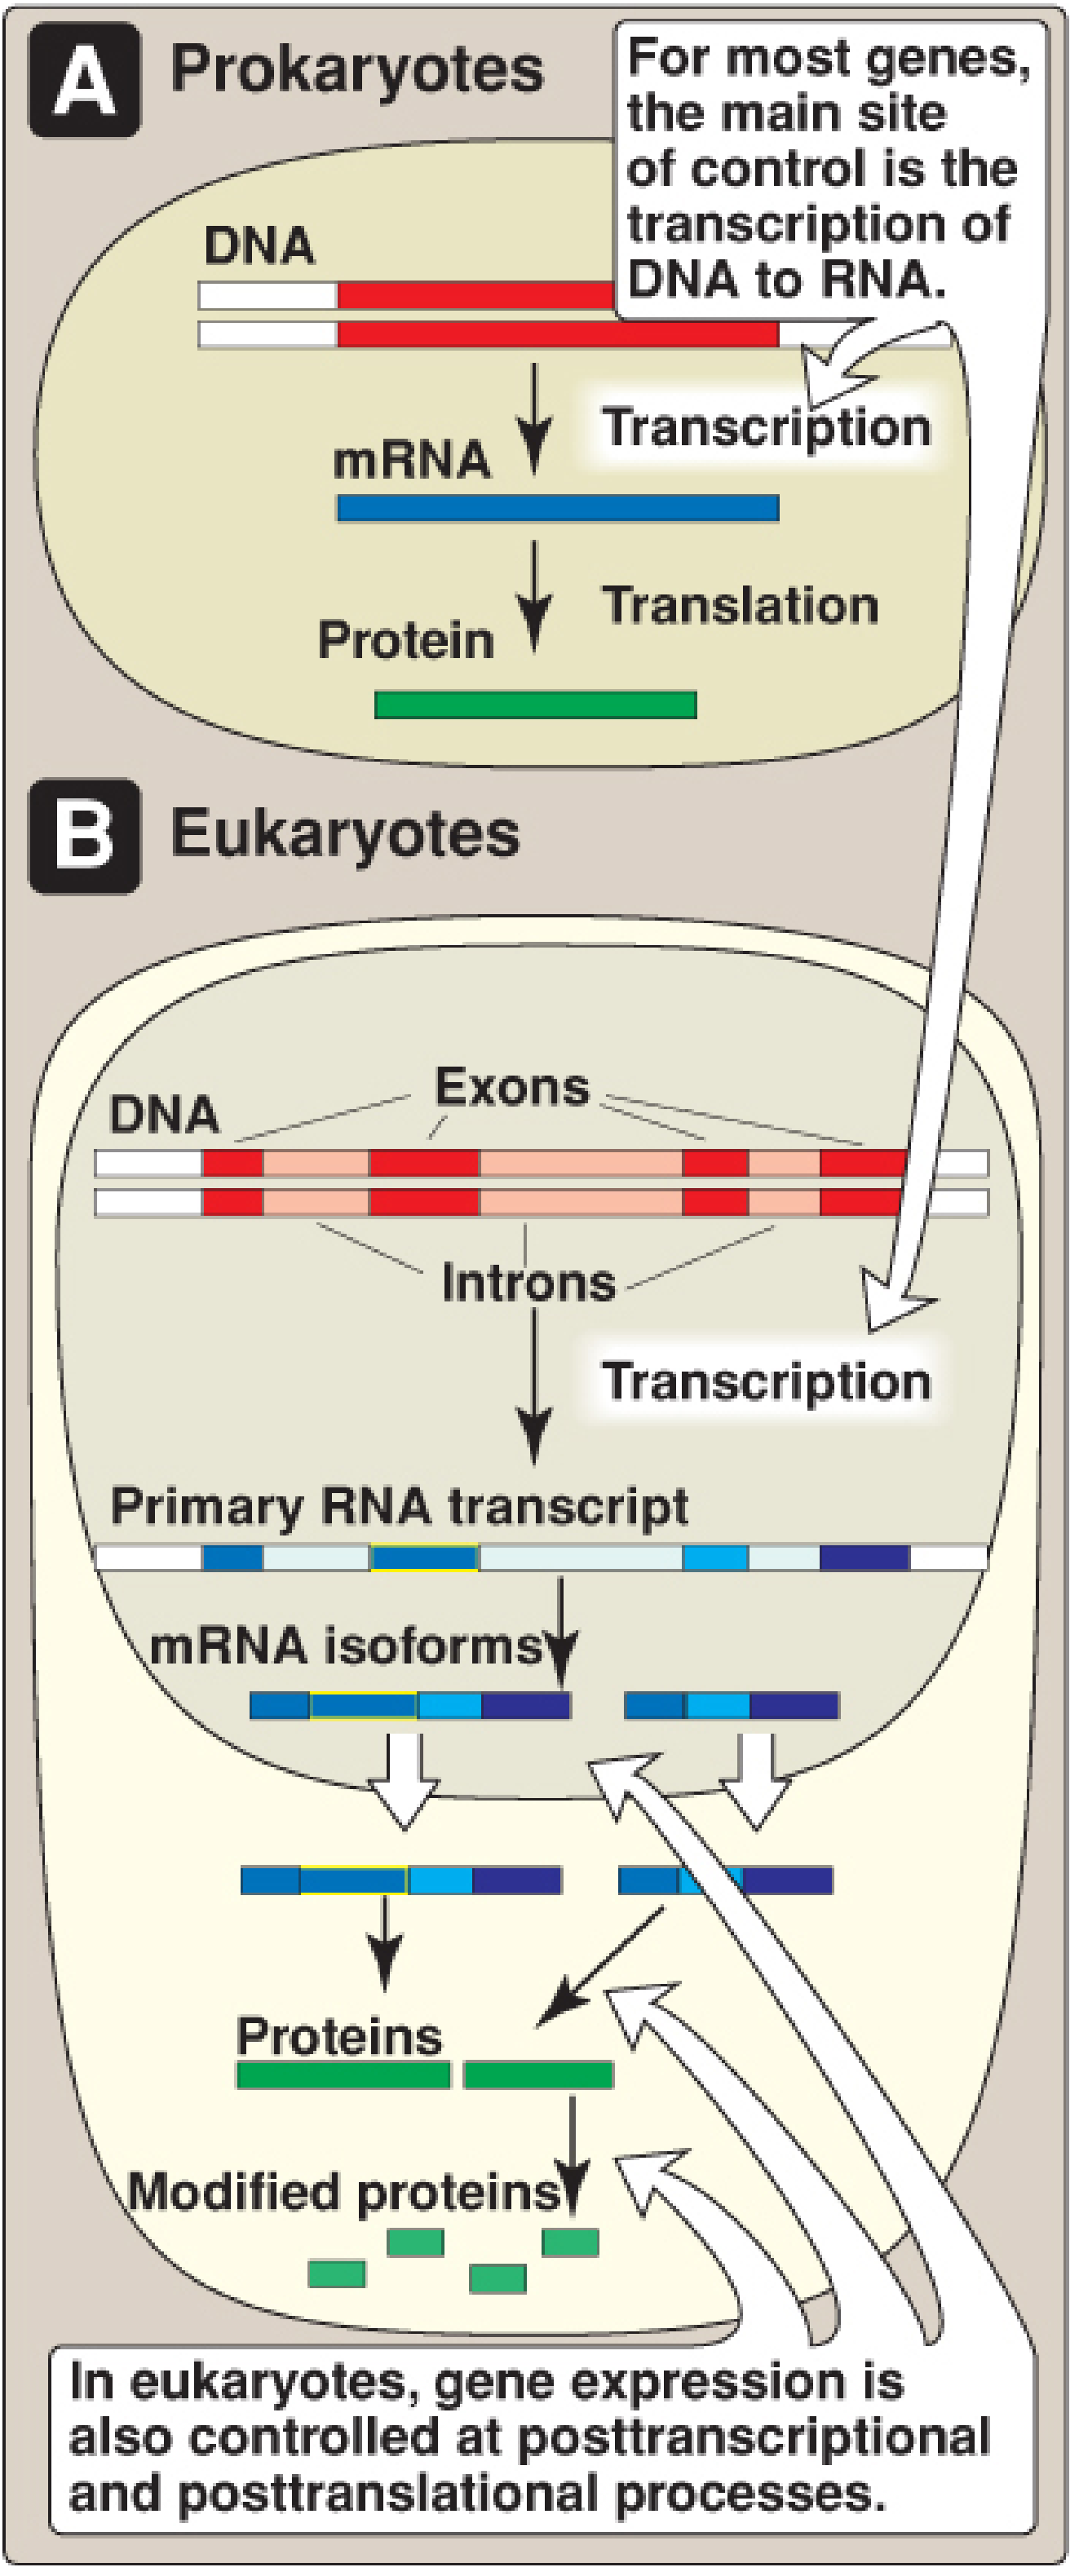
Lippincott Fig. 33.1 - In prokaryotes, transcription is the main control site. In eukaryotes, additional controls operate at posttranscriptional, translational, and posttranslational levels.
Two Types of Genes:
| Type | Description | Example |
|---|---|---|
| Constitutive ("Housekeeping") | Always expressed at a constant level | Genes for glycolysis enzymes |
| Regulated | Expressed only under certain conditions | Fibrinogen alpha chain (only in hepatocytes) |
II. THE TWO FUNDAMENTAL PLAYERS IN REGULATION
Before diving into prokaryotes vs. eukaryotes, you must understand these two concepts - they are the backbone of all transcriptional regulation:
1. Cis-Acting Elements (DNA Sequences)
- Regulatory sequences of DNA embedded in noncoding regions
- Called "cis-acting" because they influence genes on the same chromosome
- Examples: promoters, operators, enhancers, silencers, response elements
2. Trans-Acting Factors (Regulatory Proteins)
- Proteins (usually transcription factors) that diffuse through the cell and bind to cis-acting DNA sequences
- Called "trans-acting" because they can be encoded on a different chromosome from the gene they regulate
- A transcription factor encoded on chromosome 11 can regulate a gene on chromosome 6
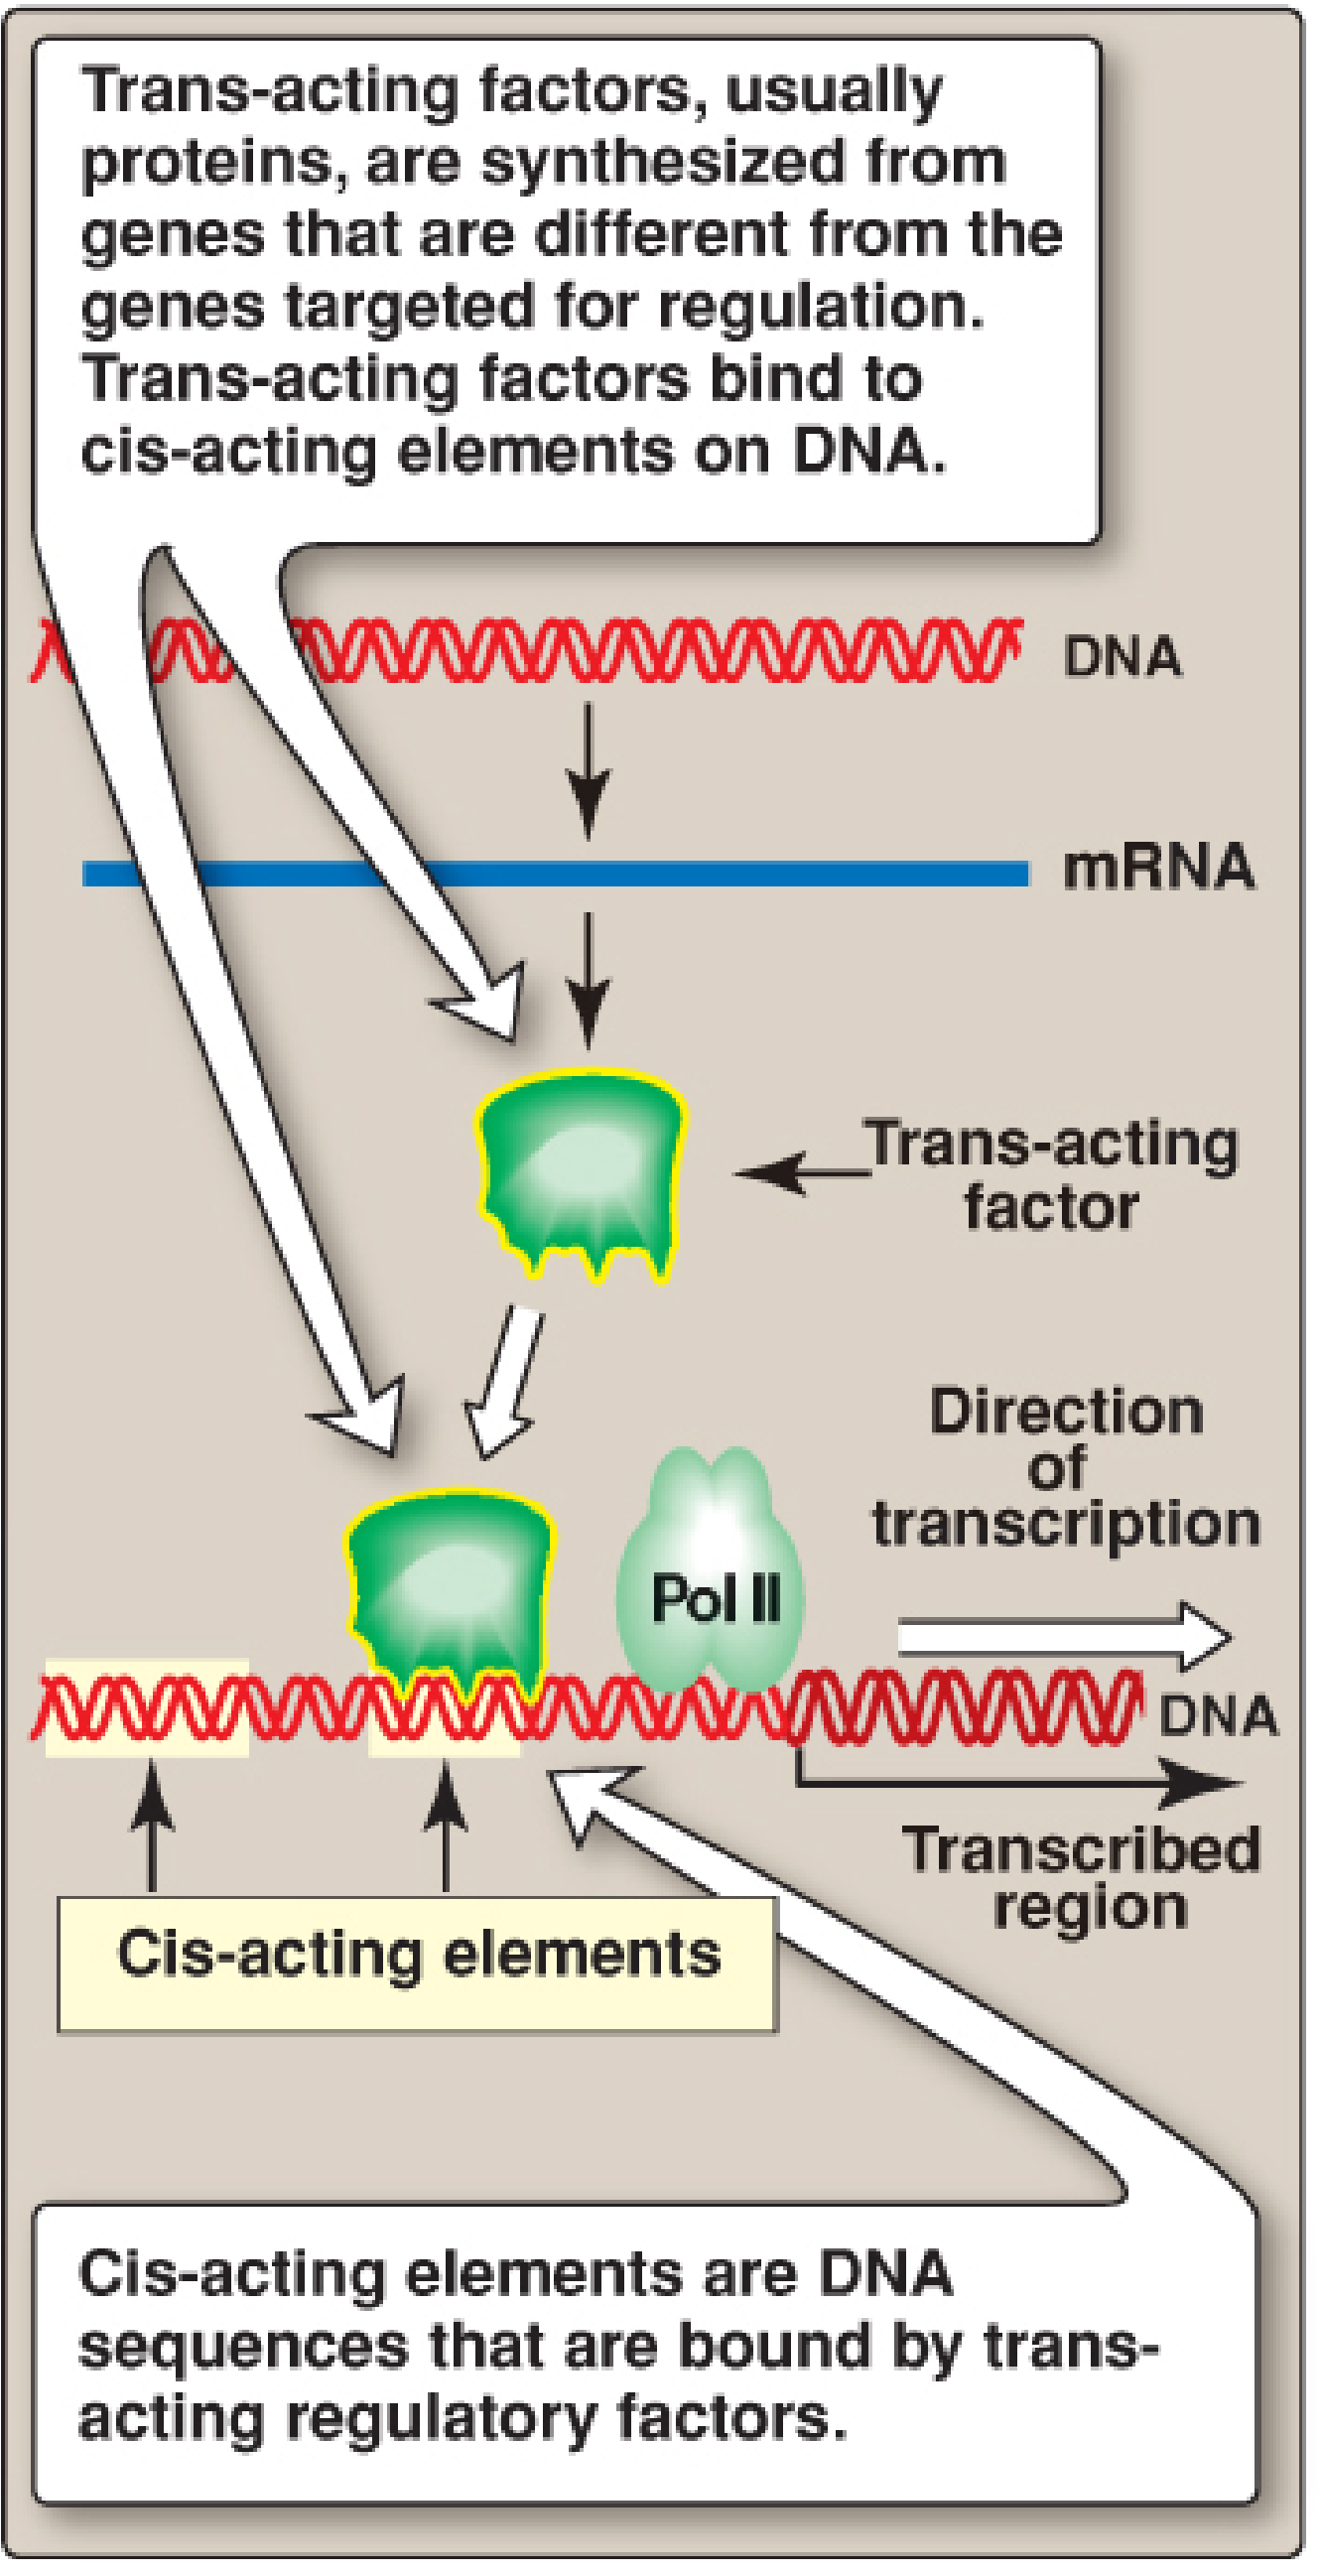
Lippincott Fig. 33.2 - Trans-acting factors are synthesized from different genes and diffuse to bind cis-acting elements on DNA, recruiting RNA Pol II.
DNA-Binding Motifs of Trans-Acting Factors:
Trans-acting factors physically grip DNA through specific structural "hands." The three most important are:
| Motif | Structure | Example |
|---|---|---|
| Zinc finger | Zn²⁺ coordinated by Cys/His residues, forming a finger-like loop | Steroid hormone receptors, Gal4 |
| Leucine zipper | Repeated leucines allow two helices to zip together and grip DNA | C/EBP, AP-1 |
| Helix-turn-helix | One helix fits into the DNA major groove | Homeodomain proteins |
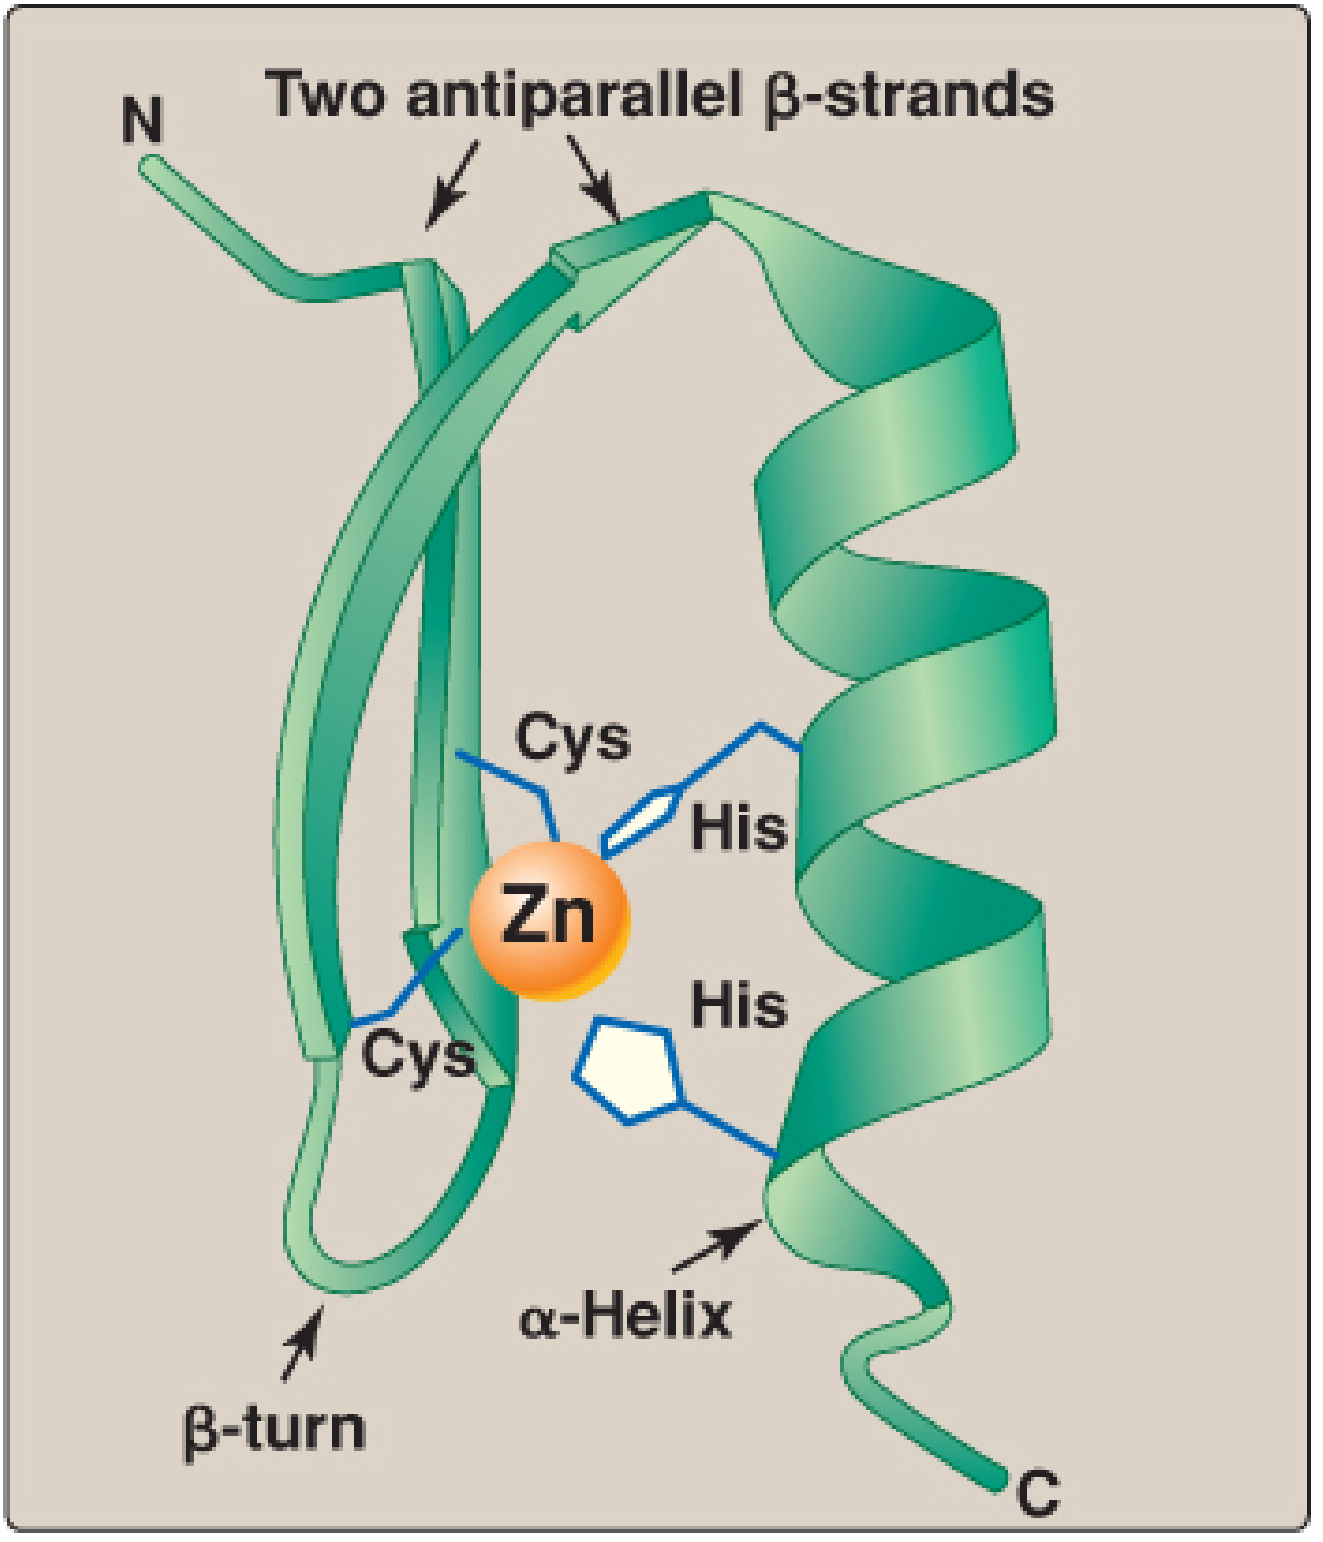
Lippincott Fig. 33.3 - Zinc finger: Zn²⁺ is coordinated by two Cys and two His residues, stabilizing the fold into antiparallel β-strands + α-helix that inserts into the DNA major groove.
III. REGULATION IN PROKARYOTES
Key Feature: The Operon
In bacteria, genes for a related metabolic pathway are clustered together on the chromosome into an operon. When transcribed, they produce a single polycistronic mRNA (one mRNA encoding multiple proteins). This allows all related genes to be switched ON or OFF together - coordinate regulation.
Structure of an operon:
5'─ [Regulatory gene] ─ [Promoter] ─ [Operator] ─ [Gene 1] ─ [Gene 2] ─ [Gene 3] ─ 3'
B. The Operator
The operator is a cis-acting DNA sequence that binds a repressor protein:
- If repressor is NOT bound → RNA pol passes freely → mRNA is made → proteins produced
- If repressor IS bound → RNA pol is blocked → no mRNA → no proteins
C. The Lactose (lac) Operon - The Classic Example
The lac operon controls catabolism of lactose in E. coli. It contains:
- lacZ → encodes β-galactosidase (hydrolyzes lactose → glucose + galactose)
- lacY → encodes permease (transports lactose into cell)
- lacA → encodes thiogalactoside transacetylase
Regulatory sites upstream of the three genes:
- Promoter - where RNA pol binds
- Operator (O site) - where repressor binds
- CAP site - where CAP-cAMP complex binds (positive regulation)
- lacI gene (has its own promoter, outside the operon) - encodes the repressor
The lac Operon Has BOTH Negative AND Positive Control:
Negative control (repressor/inducer system):
| Situation | Repressor | Operator | Transcription |
|---|---|---|---|
| No lactose | Active repressor binds operator | Blocked | OFF |
| Lactose present | Allolactose (inducer) binds repressor → repressor dissociates | Empty | Allowed |
Memory tip: Lactose is an inducible system. Lactose (via allolactose) is the inducer that removes the block.
Positive control (CAP-cAMP system):
| Situation | cAMP level | CAP-cAMP | Transcription |
|---|---|---|---|
| Glucose present | Low cAMP | CAP cannot bind | Low (glucose preferred) |
| No glucose | High cAMP | CAP-cAMP binds CAP site → ACTIVATES pol | High (lactose now used) |
Maximal transcription occurs only when: lactose IS present (operator empty) AND glucose IS absent (CAP-cAMP bound at CAP site).
This is the cell's elegant logic: "Only make lactose-digesting enzymes if lactose is available AND you don't already have glucose - your preferred fuel."
D. The Tryptophan (trp) Operon - Repressible Operon
The trp operon encodes 5 enzymes for tryptophan (Trp) synthesis. Unlike the lac operon, this is a repressible system.
Negative control:
- When Trp is scarce → repressor is inactive → genes are ON (make more Trp)
- When Trp is plentiful → Trp acts as a corepressor, binds the repressor → active repressor-Trp complex blocks operator → genes are OFF
Memory trick: lac = inducible (inducer relieves repression); trp = repressible (product represses its own synthesis). Both are examples of negative feedback.
Attenuation - Extra Layer of Trp Operon Control:
Even if the repressor doesn't fully shut down the operon, a second mechanism called attenuation can terminate transcription early.
The 5' leader region of the trp mRNA contains two Trp codons. Here's how it works:
-
Trp abundant: Ribosomes translate the leader peptide efficiently (both Trp codons satisfied) → mRNA folds into a hairpin (stem-loop) = attenuator → transcription terminates prematurely → truncated, nonfunctional peptide is degraded
-
Trp scarce: Ribosome stalls at the Trp codons (no charged tRNA-Trp available) → covering part of the mRNA prevents attenuator hairpin from forming → transcription continues → full operon is expressed
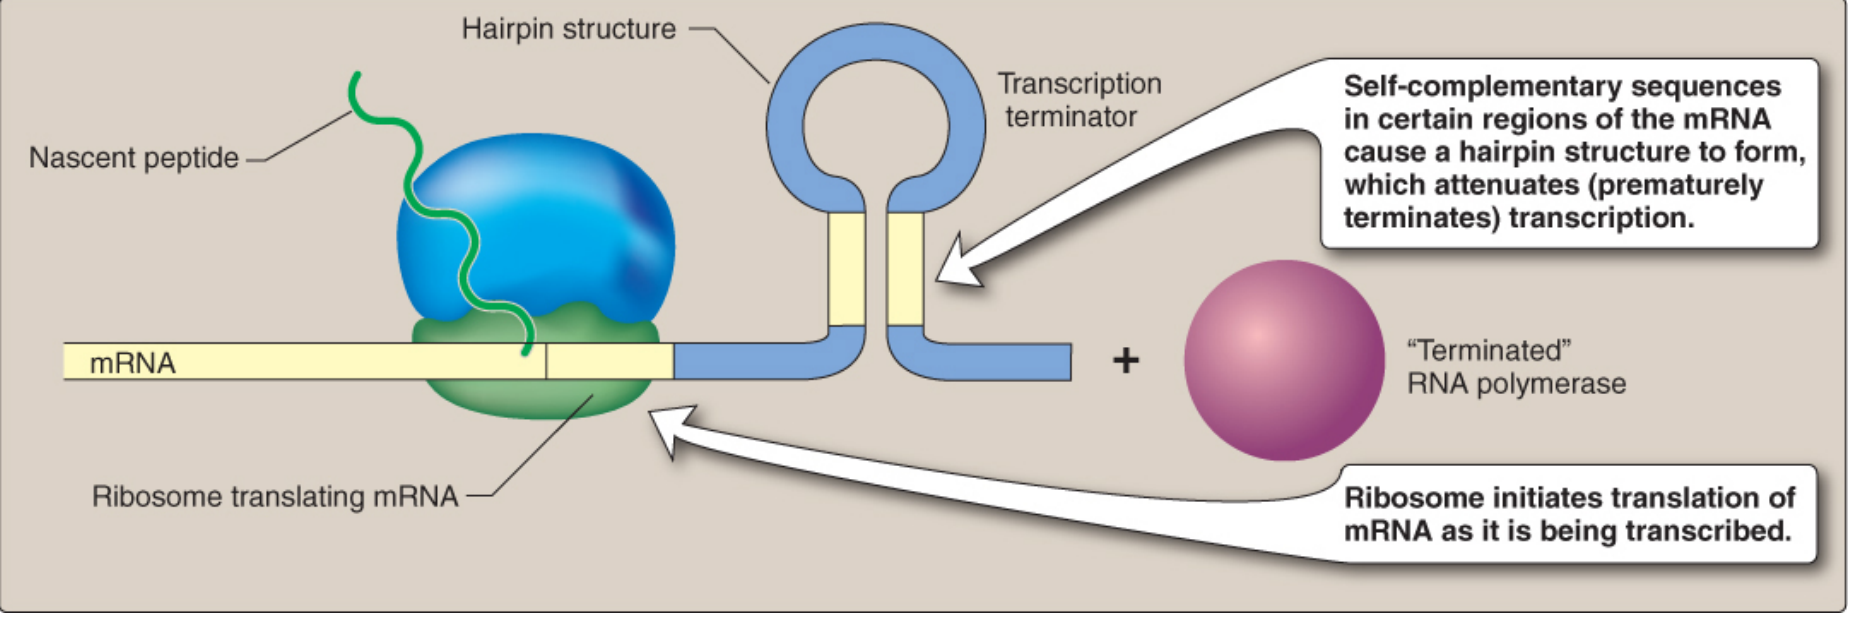
Lippincott Fig. 33.6 - When Trp is plentiful, the mRNA forms a hairpin/attenuator structure, which terminates transcription prematurely. Transcription and translation are linked in prokaryotes.
E. Stringent Response - Coordinating rRNA with Conditions
E. coli has 7 operons encoding rRNA. During amino acid starvation:
- Uncharged tRNA enters ribosome A site
- This triggers RelA (stringent factor) on the ribosome
- RelA synthesizes ppGpp (guanosine tetraphosphate) = the "alarmone"
- ppGpp binds RNA polymerase → inhibits rRNA synthesis
- Net effect: protein synthesis slows → cell conserves resources
IV. REGULATION IN EUKARYOTES
Eukaryotes need far more complex regulation because:
- Much larger, more complex genome
- Nuclear membrane separates transcription from translation
- Many different cell types must express different subsets of genes from the same DNA
- No operons - related genes may be on different chromosomes
Control is multi-layered:
DNA Access → Transcription → Pre-mRNA Processing → mRNA Stability → Translation → Protein Modification
A. Coordinate Regulation in Eukaryotes
Since related genes can be on different chromosomes, eukaryotes use specific transcription factors (STFs) to coordinate their expression.
A STF has two functional domains:
- DNA-binding domain (DBD) - physically grips the cis-acting regulatory element
- Transcription-activation domain (TAD) - recruits coactivators (e.g., histone acetyltransferases) and the general transcription machinery
This is called combinatorial control: the same TAD can recruit different proteins in different contexts, generating diverse responses.
Example 1: Galactose Circuit (Yeast)
The yeast genes for galactose metabolism are on different chromosomes, but all share an upstream activating sequence (UASgal). The STF Gal4 binds all of them:
| Galactose absent | Galactose present |
|---|---|
| Gal80 binds Gal4's TAD → TAD blocked → no transcription | Gal3 binds Gal80 → frees TAD → Gal4 activates all galactose genes |
Example 2: Hormone Response System
Steroid hormones (e.g., glucocorticoids, estrogens) are lipid-soluble and diffuse directly into cells, binding cytoplasmic receptors. The hormone-receptor complex:
- Translocates to the nucleus
- Binds to hormone response elements (HREs) - cis-acting sequences in the promoter region of target genes
- Activates transcription of ALL genes bearing that HRE, even on different chromosomes
This is why a single cortisol molecule can affect hundreds of genes simultaneously - classic coordinate regulation.
B. Chromatin Structure and Epigenetics
Eukaryotic DNA is wrapped around histones forming chromatin. This packing can physically block access to genes.
Histone Acetylation:
- Histone acetyltransferases (HATs) add acetyl groups to histone tails → loosens chromatin → DNA accessible → gene expression ON
- Histone deacetylases (HDACs) remove acetyl groups → chromatin compacts → gene expression OFF
DNA Methylation:
- Methylation of cytosine (at CpG islands near promoters) is associated with gene silencing
- Heavily methylated = gene OFF
These modifications do NOT change DNA sequence but alter gene expression - this is epigenetic regulation.
C. Posttranscriptional Regulation - After the mRNA is Made
Gene expression in eukaryotes is also regulated after transcription. The primary pre-mRNA is a rough draft that gets extensively edited:
1. Alternative Splicing
The same pre-mRNA can be spliced differently in different tissues or conditions, including or excluding different exons, producing different protein isoforms from a single gene.
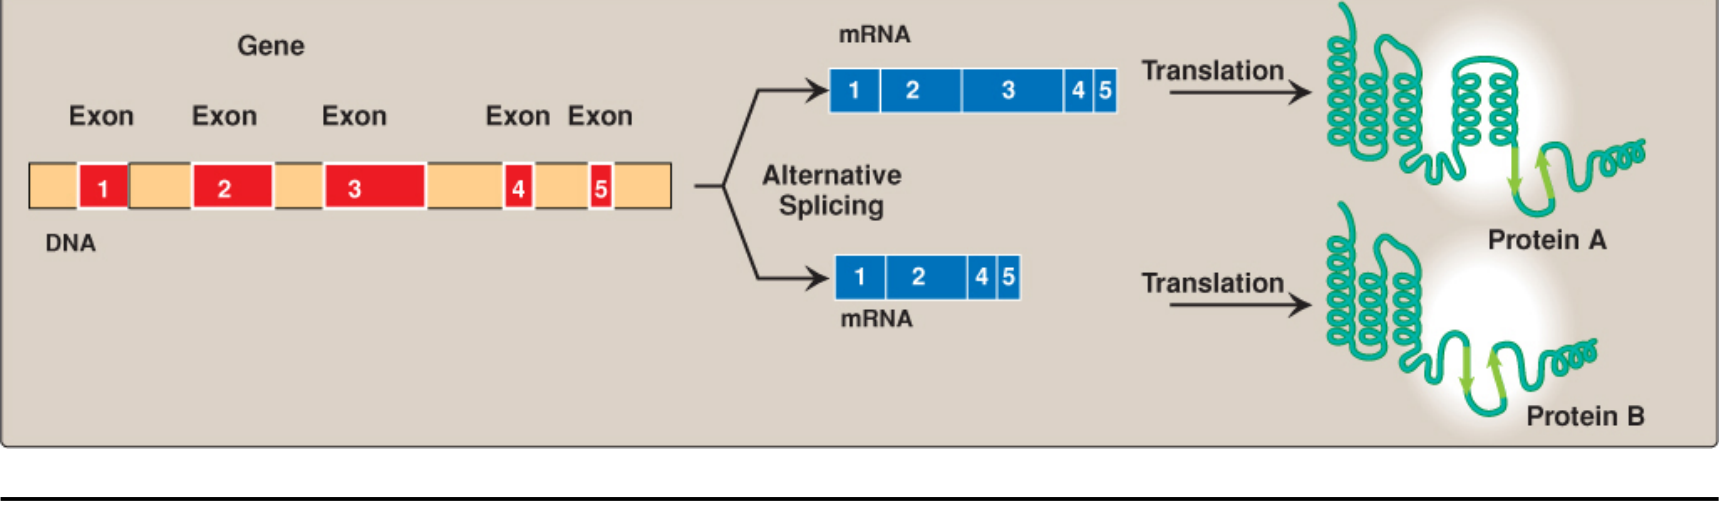
Lippincott Fig. 33.12 - Alternative splicing of the same gene's pre-mRNA produces different mRNA isoforms and therefore different proteins (Protein A vs Protein B). This helps explain how ~20,000-25,000 human genes encode over 100,000 proteins.
2. Alternative Polyadenylation (APA)
Some pre-mRNAs have multiple cleavage and polyadenylation sites. Choosing different sites alters the 3'-UTR or even the coding sequence. Classic example: production of membrane-bound vs. secreted forms of immunoglobulin M (IgM).
3. mRNA Editing
Even after processing, individual bases in an mRNA can be chemically altered.
Classic example: Apolipoprotein B (apoB)
- In the liver: full-length apo B-100 mRNA is translated → apo B-100 protein → incorporated into VLDL
- In the intestine: an enzyme deaminates C → U in the CAA codon for glutamine → CAA becomes UAA (stop codon) → shorter apo B-48 protein → incorporated into chylomicrons
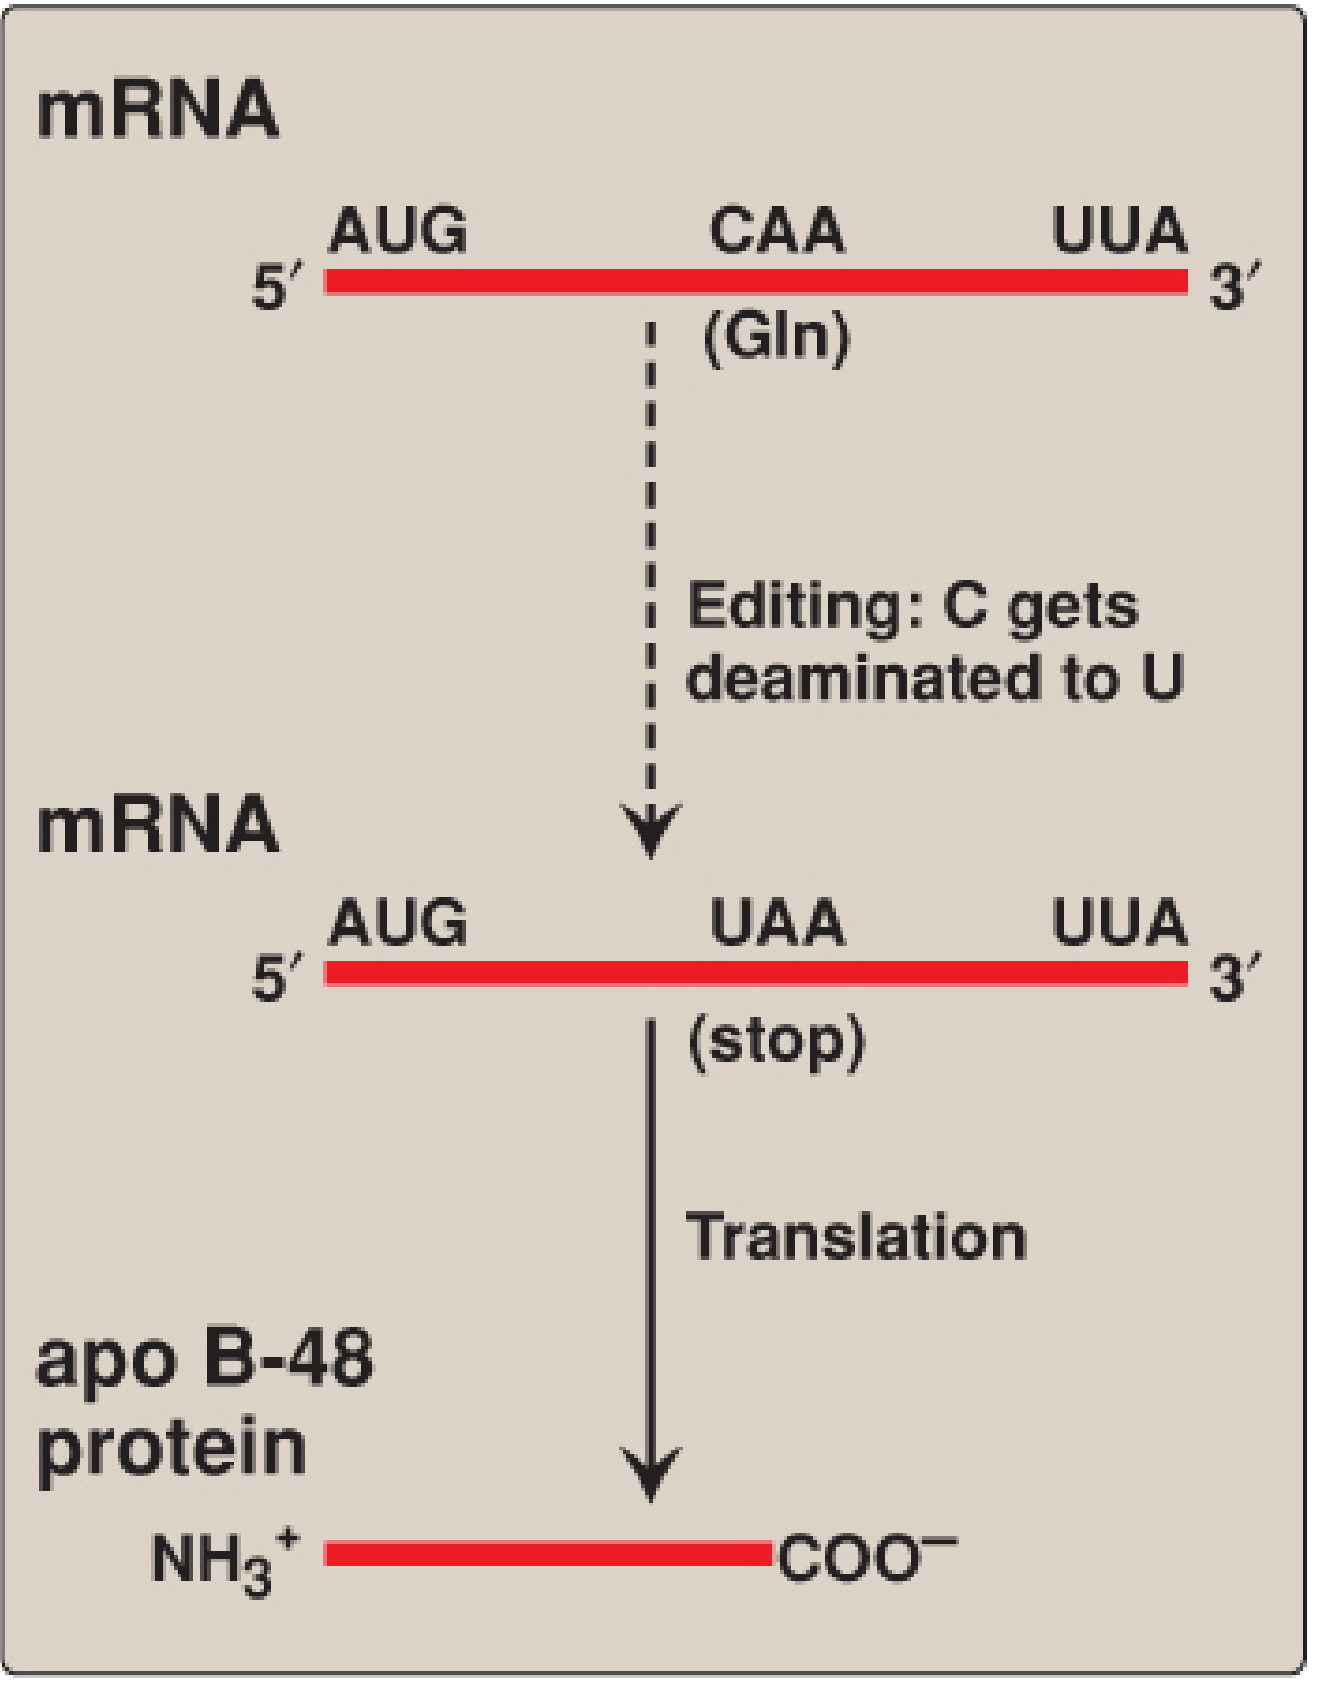
Lippincott Fig. 33.13 - In the intestine, C is deaminated to U in the apo B mRNA, changing glutamine (CAA) to a stop codon (UAA), producing the shorter apo B-48 needed for chylomicrons.
D. mRNA Stability - Controlling Lifespan
How long an mRNA survives in the cytoplasm determines how much protein can be made from it. Two key examples:
1. Iron Metabolism - Iron Responsive Elements (IREs)
| Iron Status | What Happens |
|---|---|
| Iron LOW | Iron Regulatory Protein (IRP) binds IREs in the 3'-UTR of transferrin receptor (TfR) mRNA → stabilizes mRNA → more TfR made → more iron imported |
| Iron HIGH | Iron binds IRP → IRP cannot bind IRE → TfR mRNA degraded → less iron import |
This is elegant negative feedback: low iron → stabilize the mRNA for the iron importer → bring in more iron.
2. RNA Interference (RNAi) - Gene Silencing by miRNA
MicroRNA (miRNA) are short (~22 nucleotide), noncoding RNAs that silence gene expression.
Biogenesis of miRNA:
- Genomic DNA → transcribed to long pri-miRNA (primary miRNA) in the nucleus
- Drosha (endonuclease) cleaves pri-miRNA → pre-miRNA in the nucleus
- Exportin-5 transports pre-miRNA to the cytoplasm
- Dicer (endonuclease) cleaves pre-miRNA → short double-stranded miRNA
- One strand (guide/antisense strand) loads into RISC (RNA-induced silencing complex)
- RISC-miRNA scans for complementary sequences in the 3'-UTR of target mRNA
Outcome depends on complementarity:
- Perfect match → Argonaute/Slicer (part of RISC) cleaves and degrades the mRNA
- Imperfect match → translation is repressed without mRNA degradation
Clinical relevance: In 2018, patisiran became the first approved RNAi therapeutic - a siRNA drug that silences transthyretin (TTR) mRNA to treat hereditary amyloidosis.
siRNA vs miRNA: Both use the RISC machinery, but siRNAs are exogenous (introduced from outside, used therapeutically) and require perfect complementarity; miRNAs are endogenous and work with imperfect matches.
E. Translational Regulation - Controlling at Protein Synthesis
Phosphorylation of eIF-2
Translation initiation requires the factor eIF-2 (eukaryotic initiation factor 2) in its active GTP-bound form.
Under stress conditions (amino acid starvation, heme deficiency in erythroblasts, viral infection via double-stranded RNA, misfolded proteins in RER), kinases phosphorylate eIF-2:
- Phosphorylated eIF-2 is inhibited (GDP-GTP exchange is blocked)
- Translation initiation is inhibited
- The cell halts protein synthesis to conserve resources during stress
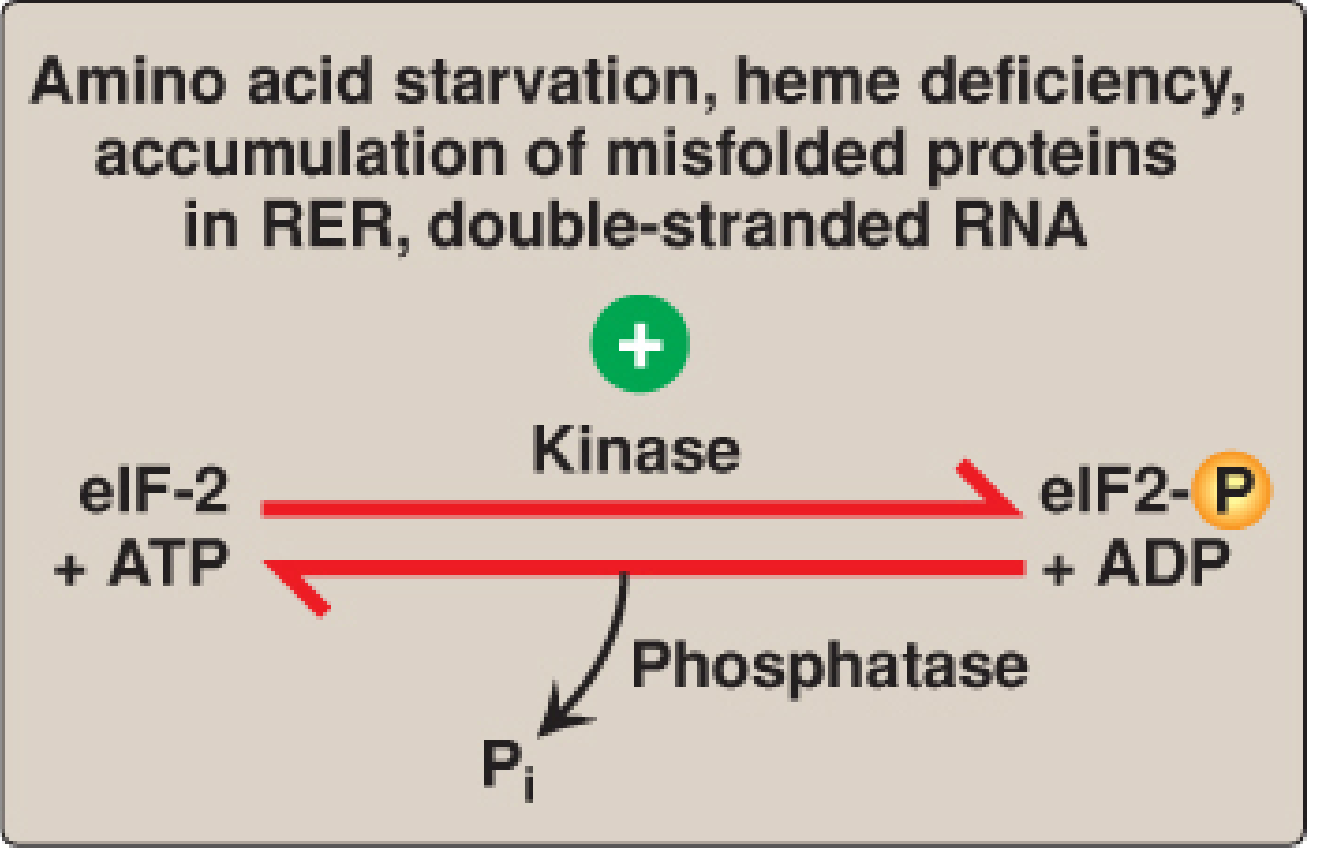
Lippincott Fig. 33.16 - Under stress (amino acid starvation, heme deficiency, viral infection, misfolded proteins), kinases phosphorylate eIF-2, blocking translation initiation. Phosphatase reverses this.
V. SUMMARY TABLE - All Levels of Regulation
| Level | Mechanism | Where | Example |
|---|---|---|---|
| Chromatin remodeling | Histone acetylation/deacetylation, DNA methylation | Nucleus | Epigenetic silencing |
| Transcription initiation | Repressor/activator binding operators/enhancers | Nucleus | lac operon, hormone receptors |
| Transcription termination | Attenuation (prokaryotes) | Nucleus (prokaryotes) | trp operon attenuation |
| Pre-mRNA processing | Alternative splicing, APA | Nucleus | Tropomyosin isoforms, IgM |
| mRNA stability | IREs, miRNA/RISC | Cytoplasm | TfR mRNA, RNAi silencing |
| mRNA editing | Base deamination | Cytoplasm | ApoB C→U editing |
| Translation | eIF-2 phosphorylation | Cytoplasm | Stress response |
| Posttranslational | Phosphorylation, proteolysis, targeting | Cytoplasm/ER | Protein activation/degradation |
VI. QUICK REVISION - HIGH-YIELD FACTS FOR EXAMS
| Fact | Detail |
|---|---|
| lac operon - inducible or repressible? | Inducible (lactose/allolactose is the inducer) |
| trp operon - inducible or repressible? | Repressible (Trp = corepressor) |
| CAP-cAMP activates what? | lac operon when glucose is absent |
| ppGpp does what? | Inhibits rRNA synthesis (stringent response) |
| Cis-acting | On the same chromosome (operators, enhancers) |
| Trans-acting | Diffusible proteins (transcription factors, repressors) |
| Zinc finger coordinates | Zn²⁺ with 2 Cys + 2 His residues |
| ApoB in intestine vs liver | B-48 (intestine, C→U edit) vs B-100 (liver, full length) |
| miRNA biogenesis enzymes | Drosha (nucleus) → Dicer (cytoplasm) → RISC |
| First RNAi therapeutic | Patisiran (2018) - treats hATTR amyloidosis |
| eIF-2 phosphorylation | Inhibits translation; triggered by amino acid starvation, viral dsRNA, heme deficiency, misfolded proteins |
| ~20,000 genes → 100,000+ proteins | Explained by alternative splicing + APA |
VII. MNEMONIC AIDS
- lac operon ON requires: "Lactose present, Glucose absent" → Let the Genes Go (LGG)
- trp operon: "Too much TRP = STOP" (Trp = corepressor = stop making more)
- Attenuation: "The ribosome stalls when Trp is small (scarce)" → no hairpin → transcription continues
- miRNA pathway: "Drosha in the Den (nucleus), Dicer in the Den's door (cytoplasm)" → both dice up RNA
- IREs rule: "Low iron = long mRNA" (IRP stabilizes TfR mRNA when iron is low)
- eIF-2 phosphorylation = STOP translating - remember the stresses: "Amino acids absent, Heme deficient, Viral dsRNA, Misfolded proteins" → A H V M
All content referenced from: Lippincott's Illustrated Reviews: Biochemistry, 8th Edition, Chapter 33, pp. 1280-1308.
This covers the entire chapter. Once you read Chapter 33 in Lippincott after going through this, you will find every section, diagram, and example immediately familiar. Would you like me to now quiz you with MCQs, create a downloadable PDF study guide, or move on to a related topic like transcription or translation?That's the complete, detailed explanation of Regulation of Gene Expression directly from Lippincott's Illustrated Reviews: Biochemistry, 8th Edition, Chapter 33.
Here's what was covered:
- Overview - what gene expression is, constitutive vs. regulated genes
- Cis-acting elements vs. Trans-acting factors - the foundation of all regulation, with DNA-binding motifs (zinc finger, leucine zipper, helix-turn-helix)
- Prokaryotic regulation - operons, the lac operon (positive + negative control), the trp operon (repression + attenuation), and the stringent response
- Eukaryotic regulation - coordinate regulation (galactose circuit, hormone response), chromatin/epigenetics, alternative splicing, mRNA editing (apoB), mRNA stability (IREs + RNAi/miRNA), and translational control (eIF-2 phosphorylation)
- Summary table across all regulatory levels
- High-yield exam facts + mnemonics
When you now open Chapter 33 of Lippincott, every figure, heading, and example will already be familiar to you. Let me know if you want:
- MCQ quiz on this topic
- A downloadable PDF study guide
- Deeper dive into any specific section (e.g., the lac operon, miRNA, epigenetics)
- Move on to a related chapter (transcription, translation, DNA replication)
This is a shared conversation. Sign in to Orris to start your own chat.